1 WHY?
Why does Brazil have no Fagales, so few Brassicaceae, and no recognized cushion plants or gypsophilous plants? Why does Mexico have more than 400 succulent Crassulaceae, while Brazil has none? Why are the tallest palms Colombian? Why have epiphytic Ericaceae failed to proliferate in the Atlantic Forest? Why? Why?
2 EXXOTAXA
Neologism: any group of species that occurs natively in South America but not natively in Brazil. Ex.: exxospecies (Koeberlinia spinosa), exxogenera (Matucana), exxofamily (Cornaceae).
3 PROBLEMATICS
Phragmites australis (Cav.) Trin. ex Steud. (Poaceae), the only Arundinoideae in South America, is cited by the VPA as native to all regions of the New World covered by the platform except Brazil (SEE). Reflora lists it as naturalized (SEE), and POWO also considers it naturalized (SEE). Why does this genus have such a strange distribution? For images of populations in French Guiana, see La Chaussette Rouge.
Does Spiranthes Rich. (Orchidaceae) really occur in French Guiana (POWO)?
Is Thismia americana N.Pfeiff. (Burmanniaceae) a fraud? Wilhelm & Rericha (The Great Lakes Botanist, 2018) discuss this hypothesis without reaching a final verdict; if confirmed, it would be an astonishing fraud and one of the largest in modern botany.
Do Cantua megapotamica Spreng. (Polemoniaceae, POWO) and Juglans brasiliensis Dode (Juglandaceae, POWO), supposedly Brazilian species, really exist?
4 BRAZILIAN NATURAL NOMENCLATURE
Nomenclature that we use in English for some Brazilian vegetation and relief formations.
igapó ‣ forest seasonally flooded by sediment-poor waters (igapó).
caatinga ‣ dry seasonal scrubland of NE Brazil (caatinga).
cerrado ‣ savannas of C Brazil (cerrado).
campinaranas ‣ northern Amazonian white-sand savannas (campinaranas).
campos rupestres ‣ rocky grasslands (campos rupestres).
campos de altitude ‣ high-altitude grasslands (campos de altitude).
cangas ‣ rocky-ferruginous grasslands (cangas).
restingas ‣ Atlantic sandy coastal shrublands (restingas).
Pico da Neblina ‣ Mount Neblina.
Serra do Aracá ‣ tepui Aracá.
5 HISTORICAL PLANTS
Wood from Calophyllum brasiliense Cambess. (Calophyllaceae), widespread across the tropical New World, was used exclusively in the production of masts and crossjacks for ships. Therefore, it became the country's first hardwood regulated by law, on 7 January 1835 (Eduzz).
Drosera magnifica Rivadavia & Gonella (Droseraceae), endemic to Minas Gerais state, is the first plant species recorded as being discovered through photographs on a social network, representing a remarkable new species of sundew from Brazil (Guinness World Records).
6 LONGEST AUTHOR CITATION
Possibly, the South American angiosperm species with the longest botanical author citation is the following, although no exhaustive documentary review has been conducted to confirm this:
Heliamphora ceracea Nerz, Wistuba, Grantsau, Rivadavia, A.Fleischm. & S.McPherson
7 REMARKABLE CITATIONS
Lindley (1849) described Lagenanthus princeps (Gentianaceae, Venezuela and Colombia, POWO) as 'one of the noblest plants in existence' (Gentian Research Network).
Judziewicz and Soderstrom, in 1990, described Glaziophyton mirabile Franch. (Poaceae) as the 'oddest bamboo in the world' (see Fernandez et al., Checklist, 2012).
According to Lytton J. Musselman, Hydnoraceae (now included in Aristolochiaceae) are 'the strangest plants in the world!' (Neotropical Hydnoraceae).
Ducke wrote of Aguiaria excelsa (Malvaceae, endemic to the Rio Negro basin): 'I am not aware of a similar seed chamber in any other plant species' (Cardoso et al., Neodiversity, 2015).
8 LOST MEDIA IN BOTANY?
From an editorial perspective, SDa considers the orchid Archivea kewensis Christenson & Jenny to be the rarest plant in Brazil, based on the exceptional scarcity of documentary evidence and the absence of confirmed wild populations. This assessment represents an editorial interpretation rather than an objective or formally established ranking of rarity; for details supporting this interpretation, see Miscellany-E. According to Plantas Raras do Brasil (UEFS, BOOK, 2009), at least another 370 species are known only from their type material, many of which have not been collected for decades or even centuries. Under the same editorial interpretation, SDa considers all these species to be equally ranked as the second rarest plants in Brazil, strictly in terms of their limited documentary records rather than their actual population sizes or geographic ranges.
9 BOTANICAL TAXONOMY IS DYNAMIC
2,875 angiosperm species were described from Brazil between 1990 and 2006 (Sobral & Stehmann, Taxon, 2009).
Many genera have undergone substantial taxonomic recircumscription, often involving the segregation of species into other genera, the recognition of previously unrecognized lineages, or extensive nomenclatural changes. Examples include Ocotea, Vriesea, Tillandsia, Orthophytum, Juncus, Paepalanthus, Chascolytrum, Paspalum, Polygala, Caesalpinia, Camptosema, Stryphnodendron, Abarema, Zizyphus, Morus, Nothofagus, Lophanthera, Licania, Hybanthus, Casearia, Phyllanthus, Tibouchina, Capparis, Cleome, Chenopodium, Mollugo, Pereskia, Opuntia, Selenicereus, Echinopsis, Loasa, Lecythis, Chrysophyllum, Pradosia, Gonolobus, Hyptis, Tabebuia, Markea and Schefflera.
Other genera have undergone substantial expansion through the incorporation of species previously assigned to separate genera, often resulting in broader generic circumscriptions. Examples include Hippeastrum, Heteranthera, Pontederia, Sedum, Alchemilla, Euphorbia, Microlicia, Miconia, Sinningia, Ameroglossum, Valeriana and Azorella.
Major taxonomic changes have also occurred in several groups, including the Androlepis Alliance in Bromelioideae (Ramírez-Díaz, J. Bromeliad Soc., 2019), the Ocotea complex in Lauraceae (Penagos Zuluaga et al., American Journal of Botany, 2021), Lobelioideae in Campanulaceae (Kagame et al., PhytoKeys, 2021), and the Espeletia clade in Asteraceae (Mavárez, Harvard Papers in Botany, 2021). In addition, extensive taxonomic restructuring has affected Portulacaceae, Petiveriaceae, Olacaceae, Saxifragaceae, and Boraginaceae, while considerable taxonomic instability persists in certain groups of South American Cactoideae.
Particularly noteworthy is the study by Chen et al. (Phytotaxa, 2015), which described 18 spp. in a family that previously comprised only 53 spp. The authors suggested that Anisophylleaceae is among the least-known angiosperm families. Likewise, Moonlight et al. (Taxon, 2018) showed that Begonia L. experienced the greatest increase in described species among flowering-plant genera, with 341 spp. described over a ten-year period. Among the study's interesting findings is the estimate that approximately 300 additional Begonia spp. remain to be described in Borneo alone.
10 RESTRICTED-RANGE PLANTS IN BRAZIL
According to Plantas Raras do Brasil (UEFS, BOOK, 2009), 2,291 rare plant species were identified in Brazil based on their restricted geographic distributions, with ranges smaller than 10,000 km².
Silva et al. (PeerJ, 2019) evaluated the distribution of 3,272 seed-plant species endemic to Brazil with geographic ranges smaller than 10,000 km². Their dataset was primarily based on the national catalogue of rare plant species in Brazil, supplemented with additional taxonomic and distributional information. The authors intersected the occurrence records of these restricted-range species with fifth-order watersheds mapped by the Brazilian government at a scale of 1:250,000 and excluded 918 species occurring in more than one watershed, resulting in a final dataset of 2,354 microendemic species.
Although geographic rarity and microendemism are closely related concepts, their definitions depend on the spatial criteria adopted. While the 2009 catalogue focused on plants with restricted geographic distributions, Silva et al. (2019) applied an additional spatial criterion, defining microendemic species as those with geographic ranges smaller than 10,000 km² and occurrences restricted to a single fifth-order watershed. Consequently, the totals of 2,291 and 2,354 should not be interpreted as directly comparable estimates, since they were obtained using different selection criteria and datasets.
11 NOTES ON RARITY
The rarity of a plant species in a given geographic context may be associated with its geographic range, population size, and habitat specificity. The table below, whose original source could not be reliably identified, illustrates eight possible combinations of these characteristics.
|
POPULATION SIZE |
| SMALL |
LARGE |
| RANGE |
WIDE |
Low Density
Longer Range
Many Habitats |
Common |
Low Density
Longer Range
Specific Habitats |
High Density
Longer Range
Specific Habitat |
| SMALL |
Restricted Range
Low Density
Many Habitats |
Restricted Range
High Density
Many Habitats |
Restricted Range
Low Density
Specific Habitats |
Restricted Range
High Density
Specific Habitats |
A plant may be considered rare because it has been collected only a few times, or because it is represented by many individuals but occupies an extremely restricted area. Under the editorial interpretation outlined in Section 8, SDa considers the orchid Archivea kewensis Christenson & Jenny to be the rarest plant in Brazil, based on the exceptional scarcity of documentary records rather than a formal assessment of population size or geographic range; for further details, see Miscellany-E. According to Plantas Raras do Brasil (UEFS, BOOK, 2009), at least another 370 species are known only from their type material, many of which have not been collected for decades or even centuries. Under the same editorial interpretation, SDa considers all these species to be equally ranked as the second rarest plants in Brazil, strictly in terms of their limited documentary records.
Searching for the term "individual" in the above-mentioned book reveals several angiosperms reported in extremely critical situations. Peritassa sadleri Lombardi (Celastraceae, Espírito Santo) and Symplocos microstyla Aranha, P.W.Fritsch & Almeda (Symplocaceae, Minas Gerais) are reported from only two individuals each, whereas Schultesia piresiana E.F.Guim. & Fontella (Gentianaceae, Bahia) and Chionanthus greenii Lombardi (Oleaceae, Minas Gerais) are reported from only a single individual. Another remarkable case is Andreadoxa flava Kallunki (Rutaceae), the sole species of its genus, reported from only one wild individual by Sambuichi (Artigos Técnico-Scientíficos Natureza & Conservação, 2008), at the Centro de Estudo do Cacau, Bahia state (CNC Flora). In terms of occupied area, noteworthy examples include Prosopanche caatingicola R.F.Machado & L.P.Queiroz (Aristolochiaceae), reported from an area of only 200 m² in Bahia state (Machado & Paganucci, Phytotaxa, 2012), and Phyllanthus eremitus Funez & Hassemer (Phyllanthaceae), reported from fewer than 30 individuals occupying just 10 m² in Santa Catarina state (Flora de Santa Catarina). According to the same book, some species were known only from cultivation, including Begonia aconitifolia A.DC. (Begoniaceae), Ruehssia carvalhoi (Morillo & Carnevali) F.Esp.Santo & Rapini (treated there as Marsdenia, Apocynaceae), Sinningia helleri Nees, and S. leucotricha (Hoehne) H.E.Moore (Gesneriaceae). None of these species is currently included in the IUCN Red List.
In a broader analysis of species richness across taxonomic groups, it is worth considering the density of species belonging to the same group within a given area. Two particularly remarkable cases can be highlighted. The first concerns the number of species in a family per 10,000 km², compared among countries or other political units. Among countries, states, or other territorial units larger than 40,000 km², Orchidaceae in Rio de Janeiro state, Brazil, may represent the highest species density worldwide, with approximately 164 species per 10,000 km², followed by Ecuador with approximately 148. These estimates are based on species counts obtained from Reflora for Rio de Janeiro and the VPA for Ecuador, divided by their respective territorial areas and expressed per 10,000 km². This ranking represents an editorial assessment based on the available data, rather than the result of an exhaustive global comparison of all territorial units.
The second concerns the density of species within a single genus. One of the most remarkable examples is the concentration of
12 GENERA OCCURRING NEAR BRAZIL
According to the taxonomic compilation presented in Synopsis of South American Angiosperms (SSAA), 1,405 angiosperm genera recorded in South America are absent from Brazil. This total reflects the taxonomic circumscriptions and distributional records adopted in the compilation and may change as new information becomes available.
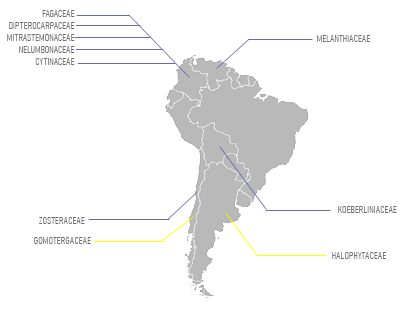
Several of these genera occur geographically close to Brazil's borders; among the most notable are Asterogyne (Arecaceae, Brittonia), Brasenia (Cabombaceae, Darwiniana), Jasarum (Araceae, GBIF), Pakaraimaea (Cistaceae, PLOS ONE), Achlyphila (Xyridaceae, NYBG, p. 12), Pyrrorhiza (Haemodoraceae, PhytoKeys), Pseudomonotes (Dipterocarpaceae, GBIF), Yasunia (Lauraceae, SEE), Steinbachiella (Fabaceae, SEE), Sarcotoxicum (Capparaceae, GBIF), Caa (Apocynaceae, Lilloa), and Argemone (Papaveraceae, Brittonia, p. 99).


| ▪ Brasenia |
| ▪ Asterogyne |
| ▪ Pakaraimaea |
| ▪ Jasarum |
| ▪ FAGALES (Myricaceae, Morella) |
| ▪ Achlyphila |
| ▪ Pyrrorhiza |
| ▪ DIPTEROCARPACEAE (Pseudomonotes) |
| ▪ Yasunia |
| ▪ Steinbachiella |
| ▪ Sarcotoxicum |
| ▪ Caa |
| ▪ PAPAVERACEAE (Argemone) |
| ▪ POLEMONIACEAE (Gilia) |
| ▪ Astragalus |
13 SELECTED DIVERSITY NOTES IN NEIGHBORING COUNTRIES
Brazil has relatively low diversity in several important groups, such as Brassicaceae, Caryophyllaceae, and the non-Amaranthoideae members of Amaranthaceae.
Based on the comparative analysis of species diversity across South American countries presented in Synopsis of South American Angiosperms (SSAA), major national centers of diversity for selected angiosperm families include Rapateaceae in Venezuela; Magnoliaceae, Arecaceae, Araceae, Heliconiaceae, Costaceae, Zingiberaceae, Brunelliaceae, Gunneraceae, Ericaceae, Gesneriaceae, Campanulaceae, and Cyclanthaceae in Colombia; Orchidaceae in Ecuador; Piperaceae, Alstroemeriaceae, Crassulaceae, Grossulariaceae, and Amaryllidaceae in Peru; Brassicaceae and Calyceraceae in Argentina; and Loasaceae in Chile. In Brazil, particularly high levels of diversity are found in Monimiaceae, Lauraceae, Bromeliaceae, Myrtaceae, Melastomataceae, and Lamiaceae. These comparisons concern species richness at the national level and reflect the taxonomic circumscriptions and distributional data adopted in the compilation.
From a morphological perspective (and within South America), some of the most notable absences from the Brazilian flora involve entire genera with distinctive biological characteristics. These include the mangrove Pelliciera (Colombia); the carnivorous Pinguicula (Venezuela to Chile); the holoparasitic genera Lennoa, Mitrastemon, and Bdallophytum (Venezuela and Colombia), and Aphyllon (Peru, Bolivia, Chile, and Argentina); the mycoheterotrophic genera Monotropa (Colombia), Degranvillea (French Guiana), Arachnitis, Tiputinia, and Triuridopsis (Peru to Argentina and Chile); the seagrasses Thalassia and Syringodium (Venezuela and Colombia); and the desiccation-tolerant dicots Blossfeldia and Clinopodium (Bolivia, Argentina, and Chile).
Other notable absences concern particular species or morphological forms rather than entire genera. These include the extremely diminutive terrestrial representatives of Viola, Begonia, and Lysipomia found in Peru, as well as giant species such as Puya raimondii (Peru and Bolivia) and Ceroxylon quindiuense (Colombia, Ecuador, and Peru). Likewise absent from Brazil are the giant-seeded representatives of genera such as Mora (Fabaceae), Pelliciera (Tetrameristaceae), and Attalea (Arecaceae), found from Colombia to Peru. In these cases, the absence refers specifically to the exceptional morphological representatives mentioned, not necessarily to the genera as a whole.
14 NOTES ON NON-NATIVE PLANTS IN SOUTH AMERICA
For a classification of non-native species according to their origin, impact, and degree of establishment, an excellent reference is Pyšek et al. (Taxon, 2004), from which the diagram below was adapted. For information on alien plants in Brazil, see RD Zenni (Rodriguésia, 2015).

SOUTH AMERICAN SPECIES INVADING OTHER REGIONS
Chapman et al. | Gymnocoronis spilanthoides DC. (OEPP/EPPO Bulletin, 2017) – documents the spread of G. spilanthoides (Asteraceae, native to southern South America) throughout the Old World.
CABI | Eichhornia crassipes (LINK) – summarizes the invasive and highly damaging nature of this South American aquatic species in many regions of the world, including historical records.
A. Rimac et al. | The Brazilian elodea (Egeria densa Planch.) invasion reaches Southeast Europe (BioInvasions Records, 2018) – documents the invasion of Croatian rivers by Egeria densa (Hydrocharitaceae).
EXOTIC SPECIES INVADING THE NEW WORLD
Alves & Roque (Check List, 2016) – first record of the African Sclerocarpus africanus Jacq. (Asteraceae) in South America (Bom Jesus da Lapa, Bahia state, Brazil).
Barbosa M.L., Alves M. & Roque N. (Rodriguésia, 2022) – first record of Heterosperma (H. ovatifolium Cav., Asteraceae) for Brazil, collected in Piatã municipality, Bahia state.
Alves et al. (Check List, 2013) – first report of the naturalization of Houttuynia cordata Thunb. (Saururaceae) in Brazil, established in Itatiaia National Park, Rio de Janeiro state.
Barcelos & Heiden – first record of the African Helichrysum foetidum (L.) Moench (Asteraceae) in South America (Canguçu and Pinheiro Machado municipalities, Rio Grande do Sul state, Brazil).
F. M. Florâncio et al. (Aquatic Botany, 2021) – detailed account of Hydrilla verticillata (L.f.) Royle in the Itaipu Reservoir (Brazil and Paraguay).
Antar et al. (Webbia, 2022) – first record of Camellia sinensis (L.) Kuntze (Theaceae) naturalized in the Brazilian Atlantic Forest.
15 CONSERVATION OF SOUTH AMERICAN PLANTS
According to a historical consultation of the IUCN Red List (SEE) conducted on 12 October 2021, 12 South American angiosperm species, representing 11 genera, were listed as Extinct (EX). These figures refer specifically to the classifications available on that date and should not be interpreted as an updated assessment of extinction in South America. Most of the listed species belong to Sapotaceae and Myrtaceae. The species recorded in this historical survey are listed below, using the names adopted in this compilation:
Sicyos villosus Hook.f. (Galapagos)
Blutaparon rigidum (A.St.-Hil.) Mears (Galapagos)
Delilia inelegans (Hook.f.) Kuntze (Galapagos)
Mida fernandeziana (Phil.) Sprague (Juan Fernández Islands, Chile)
Arachis rigonii Krapov. & W.C.Greg. (Bolivia)
Pradosia mutisii Cronquist (Colombia to NW Peru)
Casearia quinduensis Tul. (Colombia to Peru)
Campomanesia lundiana (Kiaersk.) Mattos (Brazil)
Chrysophyllum januariense Eichler (Brazil)
Myrcia neocambessedeana E.Lucas & Sobral (Brazil)
Pradosia glaziovii (Pierre) T.D.Penn. (Brazil)
Pouteria stenophylla Baehni (Brazil)
The same historical consultation identified another 10 South American angiosperm species classified as Extinct in the Wild (EW), a category indicating that a taxon is known to survive only in cultivation, captivity, or as a naturalized population outside its past range. These classifications reflect the IUCN assessments available at the time and may have been revised subsequently.
Brugmansia Pers. (Solanaceae) accounted for seven of these species in the IUCN assessments consulted in 2021. The genus was regarded as surviving exclusively in cultivation, with no confirmed herbarium records of wild individuals. According to those assessments, five species were associated with western South America, from Colombia to Chile:
B. arborea (L.) Lagerh. (IUCN).
B. aurea Lagerh. (IUCN).
B. sanguinea (Ruiz & Pav.) D.Don (IUCN).
B. versicolor Lagerh. (IUCN).
B. vulcanicola (A.S.Barclay) R.E.Schult. (IUCN).
B. insignis (Barb.Rodr.) Lockwood ex R.E.Schult. (Colombia and Brazil, IUCN).
B. suaveolens (Humb. & Bonpl. ex Willd.) Sweet (possibly native to the forests of NE Brazil, IUCN).
However, because no confirmed wild herbarium specimens were known for these species, their original geographic distributions remain uncertain. Most taxonomic sources, including the VPA, do not recognize Brugmansia as native to Brazil. This website follows Dupin & Smith (Taxon, 2018), recognizing only five species. Thus, the seven IUCN entries above are retained for historical documentation and do not represent the taxonomic circumscription adopted here.
Senecio leucopeplus Cabrera (Argentina, IUCN).
Sophora toromiro (Phil.) Skottsb. (Easter Island, Chile, IUCN).
Terminalia acuminata (Allemão) Eichler (Rio de Janeiro, Brazil, IUCN). Reports of wild individuals have raised questions about its historical EW classification (Wikiparques). However, such reports do not automatically change an IUCN category, which requires formal reassessment.
The EX and EW classifications presented above constitute a historical snapshot of the IUCN Red List as consulted on 12 October 2021. Subsequent rediscoveries, taxonomic revisions, or changes in conservation assessments may have altered the status of individual species. Accordingly, these historical classifications should be distinguished from their current conservation status.
16 DIVERSITY OF PLANTS IN SELECTED COUNTRIES
MEXICO
See Almanaque Z/BRAZIL ✕ MEXICO/COLOMBIA: BOTANY.
GUIANAS
The three Guyana countries together have 64 genera that do not occur in Brazil. None represent an absent family in Brazil. For very detailed maps of the most important sites of botanic collections in Guyana, see Hoffman (Smithsonian Plant Collection, 2014). Endemic genera marked in bold. For trees from French Guiana, see JF Molino et al. (Adansonia, 2022), who lists 1,811 spp. in 421 genera at 87 families.
GUYANA (51)
Brasenia (Cabombaceae), Chlorocardium (Lauraceae), Jasarum (Araceae), Chaubardiella, Sievekingia, Gomphihis, Eloyella, Oliveriana, Teuscheria (Orchidaceae), Potarophyton, Windsorina (Rapateaceae), Rhynchocladium (Cyperaceae, GBIF), Lutheria (Bromeliaceae), Phragmites (Poaceae), Maburea (Erythropalaceae), Whittonia (Peridiscaceae), Ceratostema (Ericaceae), Chorisepalum, Enicostema, Rogersonanthus (Gentianaceae), Didymochlamys, Duidania, Etericius, Erithalis, Maguireothamnus, Pteridocalix, Wittmackanthus, Merumea (Rubiaceae), Christopheria, Lampadaria, Pagothyra, Roogeton, Kohleria, Crantzia (Gesneriaceae), Condylidium, Quelchia (Asteraceae), Pseudanamomis (Myrtaceae), Maguireanthus, Ochthephilus (GBIF), Boyania, Phainatha, Tryssophytum, Pterogastra (Melastomataceae), Loxopterygium (Anacardiaceae), Pakaraimaea (Cistaceae), Guaiacum (Zygophyllaceae), Dystovomita, Thysanostemon (Clusiaceae, GBIF), Pibiria (Passifloraceae, SEE), Neosprucea (Salicaceae), Senefelderopsis (Euphorbiaceae).
SURINAME (16)
Chlorocardium (Lauraceae), Teuscheria, Chamelophyton, Degranvillea, Chaubardiella, Sievekingia (Orchidaceae), Lutheria (Bromeliaceae), Phragmites (Poaceae), Buxus (Buxaceae, GBIF), Chorisepalum (Gentianaceae), Kohleria, Lembocarpus, Pagothyra (Gesneriaceae), Megaskepasma (Acanthaceae), Loxopterygium (Anacardiaceae), Guaiacum (Zygophyllaceae).
FRENCH GUIANA (19)
Brasenia (Cabombaceae), Asterogyne (Arecaceae), Chamelophyton, Degranvillea, Spiranthes, Chaubardiella, Sievekingia (Orchidaceae), Lutheria (Bromeliaceae), Phragmites (Poaceae), Garciemoriana (Apocynaceae), Christopheria, Cremersia, Pagothyra, Kohleria, Lembocarpus (Gesneriaceae), Russelia (Plantaginaceae), Loxopterigyum (Anacardiaceae), Amyris (Rutaceae), Hekkingia (Violaceae).

GUYANA/SURINAME (3)
Chlorocardium (Lauraceae), Chorisepalum (Gentianaceae), Guaiacum (Zygophyllaceae)
GUYANA/FRENCH GUIANA (2)
Brasenia (Cabombaceae), Christopheria (Gesneriaceae).
SURINAME/FRENCH GUIANA (3)
Chamelophyton, Degranvillea (Orchidaceae), Lembocarpus (Gesneriaceae).
GU/SR/FG (7)
Chauberadiella, Sievekingia (Orchidaceae), Lutheria (Bromeliaceae), Phragmites (Poaceae), Kohleria, Pagothyra (Gesneriaceae), Loxopterygium (Anacardiaceae).

| ▪ Rhynchocladium |
| ▪ Jasarum |
| ▪ Ceratostema |
| ▪ Maburea |
| ▪ Potarophyton |
| ▪ Windsorina |
| ▪ Buxus |
| ▪ Asterogyne |
| ▪ Brasenia |
VENEZUELA
275 families, 2,480 genera and 15,820 species of vascular plants occur in Venezuela (Stefano, Candollea, 2009), a total that encompasses 2,964 endemic species, representing 18.7 ⁒ of the country’s vascular plant species. Total number of families, genera and species for the main vascular plant groups in Venezuela

The ten largest vascular plants families in Venezuela are listed below.

Although the total number of endemic species in Venezuela is 3,056, however, the list in above includes only the species endemic to each region, for a total of 2,994 species. Estimated number of vascular plant species and endemics in the four main geographical regions of Venezuela, in relation to the total number of taxa in each region:

Classic endemic genera from Venezuela by region are listed below.
VENEZUELAN GUYANA
Salpinctes (Apocynaceae), Achnopogon, Chimantaea, Duidaea, Huberopappus, Quelchia, Siapaea, Tuberculocarpus, Tyleropappus (Asteraceae), Brewcaria, Steyerbromelia (Bromeliaceae), Mycerinus, Tepuia (Ericaceae), Celianella (Phyllanthaceae), Neblinantha, Sipapoantha (Gentianaceae), Pyrrorhiza (Haemodoraceae), Uladendron (Malvaceae), Mallophyton (Melastomataceae), Aracamunia (Orchidaceae), Amphiphyllum, Kunhardtia, Marahuacaea, Phelpsiella (Rapateaceae), Aphanocarpus, Cephalodendron, Coccochondra, Coryphothamnus, Duidania, Holstianthus, Yutajea (Rubiaceae), Apocaulon, Rutaneblina (Rutaceae), Achlyphila (Xyridaceae).
ANDES
Coespeletia, Carramboa, and Ruilopezia - all three segregated from Espeletia, Freya (Asteraceae), Stalkya (Orchidaceae).
COASTAL CORDILLERA
Margaritolobium (Fabaceae), Rojasimalva (Malvaceae), Llewelynia (Melastomataceae) and Neoblakea (Rubiaceae).
Llanos no has endemic genera. The genera Salpinctes (Apocynaceae), Tyleropappus (Asteraceae), Tepuia (Ericaceae), Margaritolobium (Fabaceae), Llewelynia (Melastomataceae), Cephalocarpus, Yutajea (Rubiaceae) are not recognized in SSAA. Neoblakea (Rubiaceae) now occur also in Ecuador. Neblinantha and Sipapoantha (Gentianaceae) occur in northern Brazil. Coespeletia, Ruilopezia (Asteraceae), Brewcaria and Steyerbromelia (Bromeliaceae) also occur in Colombia (the last also in Brazil). Quelchia (Asteraceae) also occur in Guyana. On the other hand, Orinoquia (Apocynaceae), Dasyandantha, Tamananthus (Asteraceae) and Autana (Podostemaceae) are absent from work but recognized as endemic to the country by the SSAA.
COLOMBIA
See Almanaque Z/BRAZIL ✕ MEXICO/COLOMBIA: BOTANY.
PERU
For a list of all vascular plants in Peru, see PERU CHECKLIST, or their ADVANCED SEARCH, both from MOBOT.
BOLIVIA
For a list of all vascular plants in Bolivia, see Bolivia Checklist.
PARAGUAY
374 taxa from 52 families and 162 genera are endemic Paraguay (Peña Chocarro & De Egea, Phytotaxa, 2018). Paraguay Biodiversidad is an excellent natural album of plants collected in their native state in Paraguay.
PARAGUAY/URUGUAY
According to the data provided by this blog, Paraguay and Uruguay have 63 genera of angiosperms absent in Brazil across 31 families, 30 of the genera only in Paraguay, 25 only in Uruguay and 8 in both. Furthermore, 4 of the families do not occur in Brazil: Montiaceae, Polemoniaceae, Frankeniaceae e Papaveraceae. Montia fontana L. posssibly introduced in Uruguay (Flora del Cono Sur/Montia fontana).
 The most remarkable of this genera is Astragalus L. (Fabaceae), the second largest genus worldwide; in Uruguay occur A. distinens Mackloskie, known from NE Argentina and Colonia, Montevideo, Río Negro, San José and Soriano departaments in SE Uruguay, mostly in sandy, open grasslands places.

MOZAMBIQUE
The checklist of angiosperms of Mozambique includes 7,099 taxa (5,957 species, 605 subspecies, 537 varieties), belonging to 226 families and 1,746 genera. There are 6,804 angiosperms, 257 pteridophytes, and 38 gymnosperms. A total of 6,171 taxa are native to Mozambique, while 602 are introduced and the remaining 326 taxa were considered as uncertain status. The endemism level for Mozambique’s flora was assessed at 9.59 ⁒, including 278 strict-endemic taxa and 403 near-endemic. 58.2 ⁒ of taxa are herbaceous, while shrubs and trees account respectively for 26.5 ⁒ and 9.2% ⁒ of the taxa. The checklist also includes ferns (3.6 ⁒), lianas (1.7 ⁒), subshrubs (0.5 ⁒) and cycads (0.3% ⁒). Fabaceae, Poaceae and Asteraceae are the three most represented families, with 891, 543 and 428 taxa, respectively (Délcio Odorico et al., PhytoKeys, 2022).
CHINA
According to an overview of higher plant diversity in China, China has 35,112 native species of higher plants belonging to 3,818 genera and 454 families. Among them, there are 3,045 bryophyte species in 602 genera and 151 families, 2,124 pteridophyte species in 176 genera and 38 families, 227 gymnosperm species in 37 genera and 8 families, and 29,716 angiosperm species in 3,003 genera and 257 families (Lisong Wang, Yu Jia, Xianchun Zhang, Haining Qin, Biodiv Sci, 2015).
Comparisons with recent estimates of global species diversity suggests that the species diversity of Chinese of the global totals of bryophytes (18%), pteridophytes (17%), gymnosperms (22%) and angiosperms (11%) account for. A total of 212 genera are endemic to China with 7 bryophytes, 2 pteridophytes, 7 gymnosperms, and 196 angiosperms. A total of 17,439 species are endemic to China including 524 bryophytes, 840 pteridophytes, 115 gymnosperms, and 15,960 angiosperms.
The top 10 families with highest species diversity are Asteraceae (227g/2,315 species), Poaceae (215/1,787), Fabaceae (141/1,631), Orchidaceae (205/1,556), Lamiaceae (103/975), Ranunculaceae (38/957), Rosaceae (53/954), Cyperaceae (32/871), Ericaceae (22/841), and Rubiaceae (94/696).
The top 12 families with highest endemic genera are Gesneriaceae (26 genera), Asteraceae (18), Orchidaceae (14), Lamiaceae (11), Apiaceae (9), Brassicaceae (9), Apocynaceae (6), Poaceae (6), Melastomataceae (5), Boraginaceae (4), Rubiaceae (4), and Ranunculaceae (4).
The top 10 genera with highest species diversity are Rhododendron (588), Carex (537), Astragalus (420), Pedicularis (363), Corydalis (357), Primula (310), Saussurea (293), Salix (279), Impatiens (274), and Gentiana (255).
The top 10 genera with highest endemic species are Rhododendron (433), Pedicularis (283), Carex (273), Corydalis (258), Astragalus (237), Impatiens (234), Primula (222), Berberis (209), Elatostema (207), and Saussurea (196). Diversity bearing with more than 5,000 species among the seven Chinese provinces is as follows: Yunnan (15,900), Sichuan (10,374), Tibet (7,629), Guangxi (7,399), Guizhou (6,405), Guangdong (5,498) and Taiwan (5,290).
Among the 17 mega-diversity countries China is ranked the fourth when ordered by total species diversity. 1,038 spp. of angiosperms was described in China between 2013 to the end of 2018 (Cai et al., PhytoKeys, 2019).
NEW GUINEA
World’s largest tropical island and has fascinated naturalists for centuries. Home to some of the best-preserved ecosystems on the planet and to intact ecological gradients — from mangroves to tropical alpine grasslands — that are unmatched in the Asia-Pacific region, it is a globally recognized centre of biological and cultural diversity. So far, however, there has been no attempt to critically catalogue the entire vascular plant diversity of New Guinea. Here we present the first, to our knowledge, expert-verified checklist of the vascular plants of mainland New Guinea and surrounding islands. Our publicly available checklist includes 13,634 species (68 ⁒ endemic), 1,742 genera and 264 families - suggesting that New Guinea is the most floristically diverse island in the world. Expert knowledge is essential for building checklists in the digital era: reliance on online taxonomic resources alone would have inflated species counts by 22 ⁒. Species discovery shows no sign of levelling off, and we discuss steps to accelerate botanical research in the ‘Last Unknown’. (Cámara-Leret et al., Nature, 2020).
AUSTRALIA
See FloraBase of the Western Australia.
17 NEW WORLD CROPS
Three of the world's eight most produced primary agricultural crops, ranked by production volume in metric tonnes, are native to the New World: maize (2nd), a monocot originating in Mesoamerica; and potato and cassava (7th and 8th, respectively), both originating in South America. These rankings are based on global agricultural production data for 2024 (FAOSTAT, FAO).
 The other five crops among the world's eight most produced are sugarcane, rice, and wheat (Poaceae), all originating in the Old World; soybean (Fabaceae), native to Asia; and oil palm (Arecaceae), native to tropical Africa. In this ranking, oil palm production refers to harvested fruits rather than processed palm oil.
Sugarcane is the world’s largest cultivated cash crop with its incredible ability to synthesize and accumulate sucrose in its stem; present-day sugarcane is a man-made hybrid clone produced from Saccharum officinarum L. (Indonesian Archipelago, absent in the natural wild conditions but was grown and maintained for a long time by the island natives) and S. spontaneum L. (Morocco to Australia, Kazakhstan to Java) with a few genes incorporated from Saccharum ✕ sinense Roxb. (∼S. barberi, Indian cane and Chinese cane, contested taxa) and to a limited extent from S. robustum E.W.Brandes & Jeswiet ex Grassl (Wallacean cane), all from tropical Asia to Oceania (KSD Babu et al, Genetic Resources and Crop Evolution, 2022).
Hexaploid bread wheat (Triticum aestivum L., AABBDD) — which archaeological evidence places as originating in SE Turkey — contains three distinct genomes, each derived from a different diploid species. Initially, wild T. urartu Thumanjan ex Gandiljan (AA) hybridized with wild Aegilops speltoides Tausch (BB), followed by a chromosome doubling event that produced the fertile tetraploid wheat, T. turgidum L. (AABB). Following the domestication of wild emmer (T. turgidum) in the Fertile Crescent, it hybridized with the wild diploid A. tauschii Coss. (DD), giving rise to hexaploid wheat (AABBDD). Due to its high nutritional value and adaptability as a primary calorie source, hexaploid wheat spread globally along diverse trade routes. Centuries of cultivation and selective breeding across varied geographical regions ultimately shaped modern bread wheat. Among diploids, einkorn wheat (T. monococcum L.) is considered the earliest domesticated hulled wheat, with historical records dating its domestication to 12,000–8,500 years ago during the Pre-Pottery Neolithic period. Additionally, the cultivated tetraploids T. turgidum subsp dicoccum (emmer wheat) and T. turgidum subsp durum (durum wheat) both evolved from wild ancestors (S.Gohar et al., Frontiers in Genetics, 2022).
Asian cultivated rice Oryza sativa L. was domesticated from the wild rice species O. rufipogon Giff. — the domestication process began around 9,000 years ago in China, possibly in the Yangtze valley, besides the wider range of this species from India to Australia (POWO). There, early communities selected for rice plants with beneficial traits, such as enhanced seed/fruit size, better flavor, and resistance to diseases, pests, and environmental stresses (Fornasiero, Wing & Ronald, Current Biology, 2022).
Cultivated soybean (Glycine max subsp max) appears to have been domesticated from its wild relative G. max subsp soja (Siebold & Zucc.) H.Ohashi 6,000–9,000 yrs ago in China. Although the exact site of origin of soybean is unknown, S China, the Yellow River valley of central China, NE China, Korea and Japan have been identified as candidate regions where soybean could have been domesticated. Chinese literature has indicated that soybean was cultivated during the Shang dynasty from 1,700 to 1,100 BC. Clearly, soybean has been cultivated much longer than the historical evidence indicates. It is commonly accepted that the current cultivated soybean was domesticated from G. max subsp soja. However, some works have suggested that soybean was domesticated from a common ancestor of these two Glycine subspecies, based on a calculated divergence time (MT Kim et al., Breeding Science, 2012).
1. MAIZE (Zea mays L., Poaceae| 1,148 M tons in 2021)
Maize domestication began in SW Mexico ∼9,000 calendar years before present and humans dispersed this important grain to South America by at least ∼7,000 years as a partial domesticate. South America served as a secondary improvement center where the domestication syndrome became fixed and new lineages emerged in parallel with similar processes in Mesoamerica. Later, Indigenous cultivators carried a second major wave of maize southward from Mesoamerica (∼2,000 yr), hybridizing with long-established landraces from the first wave, and that some of the resulting newly admixed lineages were then reintroduced to America Central. Direct radiocarbon dates and cob morphological data from the rock shelter suggest that more productive maize varieties developed between ∼4,300 and ∼2,500 BP. (SEE).

2. POTATO (Solanum tuberosum L., Solanaceae | 370.4 M tons in 2021)
Cultivated potatoes came from the wild species extensively cultivated in the Andean region (Peru, N Argentina and Bolivia) — the domestication of cultivated potato occurs some 8,000 to 10,000 years ago, from diploid wild species (2n = 2✕ = 24). S. stenotomum (2✕) was the first domesticated potato and considered as the descendant of diploid (2✕) wild species. Andean cultivated tetraploids (S. tuberosum group Andigena; 2n = 4✕ = 48) were produced as a result of autopolyploidization of early diploid landraces S. tuberosum groups Stenotomum [2✕] and Phureja [2✕]. The domestication of potato from wild species S. brevicaule complex encompasses the selection for underground traits like large tubers with diverse shapes and colour, shorter stolon and reduced bitter taste due to tuber glycoalkaloids. The oldest record of potato consumption is from the site called Jisk'a Iru Muqu, in the Western Titicaca Basin in the Andes mountains of Peru, in 3,400 B.C (NYTimes).

Potatoes were introduced to Europe from the Americas by the Spanish in the second half of the 16th century. Today they are a staple food in many parts of the world and an integral part of much of the world's food supply. As of 2021, potatoes were the world's seventh-largest food crop after maize (corn), wheat, rice, milk and oil palm; following millennia of selective breeding, there are now over 5,000 different types of potatoes. Over 99 ⁒ of potatoes presently cultivated worldwide descend from varieties that originated in the lowlands of south-central Chile (Wikipedia).
3. CASSAVA (Manihot esculenta Crantz, Euphorbiaceae | 303.6 M tons in 2021)
With the species Manihot esculenta subsp flabellifolia (Pohl) Ciferri recognized as the strongest candidate for the botanical progenitor of domesticated manioc, both the species 'geographical evolution' and 'its initial agricultural cultivation' are estimated to have taken place in the central Brazilian savannas (cerrado) south of the Amazon rainforest, from where the crop spread during the early Holocene — possibly as early as 10,000 years ago and certainly by 7000 BC — becoming readily available across most Neotropical habitats by the mid-Holocene, at least 6,500 years ago (Latin America Antiquity) Cassava was domesticated only once, in southern Amazonia, and that no historical hybridization occurred between cassava and wild relatives in northern Amazonia (Mol. Phyl. Evol., 2009).

Cassava starches have been identified in NC Colombia by approximately 7,500 years ago, and in Panama at Aguadulce Shelter, about 6,900 years ago. Pollen grains from cultivated cassava have been found in archaeological sites in Belize and Mexico's Gulf coast by 5,800–4,500 bp, and in Puerto Rico between 3,300 and 2,900 years ago. Thus, scholars can safely say that the domestication in the Amazon had to happen before 7,500 years ago (ThoughtCo).
18 LIST OF LINKS
IMAGE DATABANKS
Gymnosperm Database (Gymnosperms)
Manual das Palmeiras do Acre, Brasil (Arecaceae)
Encyclopedia of Bromeliads (Bromeliaceae)
Orquídeas do Rio Grande do Sul (Orchidaceae)
Plantas do Brasil: Leguminosa - Fabaceae (Fabaceae)
Euphorbia PBI (Euphorbia)
Euphorbia nos EUA (Euphorbia)
Malpighiaceae Genera (Malpighiaceae)
Malvaceae Info (Malvaceae)
e-Monograph of the Caricaceae (Caricaceae)
MelNet (Melastomataceae)
The Evening Primrose Family (Onagraceae)
67° CNBOT (Loasaceae)
NYBG/Lecythidaceae (Lecythidaceae)
Luteyn/Peñalosa: NYBG (Ericaceae)
CactiGuide (Cactaceae)
Martine Deshoges - PDF (Taxonomy of Cactaceae)
Caryophyllales (Caryophyllales)
Pilger (Santalaceae)
Calió, 2013 (Gentianaceae)
Cole & Tolke (Apocynaceae)
PLATFORMS
iNaturalist - repository of photos from different authors validated by peer recognition, rarely from herbarium, which includes animals, plants and fungi from all over the world; source of rare images and some unpublished on the open search of Google with searches allowed at various taxonomic levels and even by popular names! It has the disadvantage of, in some groups, an excess of samples cultivated in gardens and orchards.
SpeciesLink - remarkable Brazilian database dealing with animals, plants and fungi with records in herbaria or not; the search can be refined by living material and botanical family, which leads to incredible images, a good part of photo libraries, some of species that are not seen on the open internet - since the images on the platform are not traceable by Google. It rarely includes cultivated, garden, or anthropized types.
NEOTROPICAL PLANTS - IMAGE DATABASE KEW - images of various groups, mainly taken in Mato Grosso and Minas Gerais (but also Panama, Bolivia and Peru), organized by family; a disadvantage is few images per species, sometimes just a detail of the plant.
Flora de Santa Catarina - excellent work that has been showing the world a surprising diversity in this beautiful Brazilian state; many images with low contrast; includes many species in anthropic environments. It has already supported botanical publications.
FLORA DIGITAL DO RIO GRANDE DO SUL - records of plants collected in Rio Grande do Sul; unfortunately most are of poor quality.
FLORA DIGITAL DO RIO GRANDE DO SUL E SANTA CATARINA - blogspot apparently abandoned, with many records of plants from southern Brazil.
Álbuns de Alex Popovkin - very detailed collection of numerous plants (and also animals) from the Atlantic Forest in northeastern Bahia, some of excellent quality. It has already supported botanical publications.
Flore de Guyane - from French Guiana; some images with unfavorable lighting but on average second best page to view after SpeciesLink; offers the invaluable advantage of chronologically organized posts.
La Chaussette Rouge - one of the richest easy-access pages in the French Guiana Amazon; navigation without bureaucracy, but not chronologically organized.
Guia Igapó - brings many records of plants collected in the upper Rio Negro, Amazonas, but few bring the plant in a natural environment, and it seems abandoned.
Paraguay Biodiverso - light and remarkable page with beautiful records from the Chaco country; it sins for having many unidentified taxons.
Fotos de Flora Nativa e Adventícias de Uruguay - showing with high quality several species from the neighboring platine country; brings records in Uruguay of three families that do not occur in Brazil: Polemoniaceae, Montiaceae and Papaveraceae.
PHOTO CATALOG
Phytoimages - spectacular in natura photo catalog, although not synced with APG IV.
PlantSystematic - very similiar to link above.
Flora of the World - shows pictures of plants from all over the world, organized by family.
Ukrbin - page of Ukrainian origin, brings many excellent images from various parts of the world, especially E Europe, but few in South America.
Botany.cz/Venezuela, Roraima - several images for plants of E Venezuela region.
Roraima Tepui - some images of plants in Mount Roraima in Venezuela.
EXPEDITIONS
Bromeliário Imperialis - promotes expeditions in eastern Brazil, especially in Bahia state; good source of Bromeliaceae images.
Vertical Garden - Patric Blanc - one of the largest panels of beautiful botanical images in existence; focused on species in their original habitat across the planet.
Expedição Fitogeográfica - makes expeditions throughout South America, especially in the Center-South region of the country; little precision in species identification.
Fábio Colombini - a remarkable album of extremely beautiful Brazilian landscapes, but it does not have identifications and seals the images with an immense watermark.
VIRBOGA - brings many interesting images from around the world; in the case of Brazil, it has a great focus on the Northeast, but includes many anthropized records; also has a watermark.
19 BIBLIOGRAPHY for publications about botany, mainly taxonomy, we have a wide range of references.
Phytotaxa
PhytoKeys
Molecular Phylogenetics and Evolution
Taxon
Systematic and Biodiversity
Novon
Brittonia
Kew Bulletin
Botanical Journal of the Linnean Society
Systematic Botany
Nordic Journal of Botany
Annals of the Missouri Botanical Garden
Havard Papers in Botany
Acta Botanica Brasilica
Biota Neotropica
Rodriguesia
Lankesteriana
Webbia
CANDOLEA
American Journal of Botany
Peerj
Edinburgh Journal of Botany
Peerj - Plant Sciene Taxonomy
Feddes Repertorium
Phytologia
Willdenowia
Bradleya
Lilloa
Darwiniana
Caldasia
Neodiversity
PlantNow
Plant Diversity
Aquatic Botany
Molecular Plant
Organisms Diversity & Evolution
Rheedea
Hacquetia
Adansonia
Plant Ecology and Evolution
Plant and Fungal Systematics
The Botanical Review
Brazilian Journal of Botany
European Journal of Taxonomy
International Journal of Plant Sciences
Aroideana
Taiwania